1. Introduction
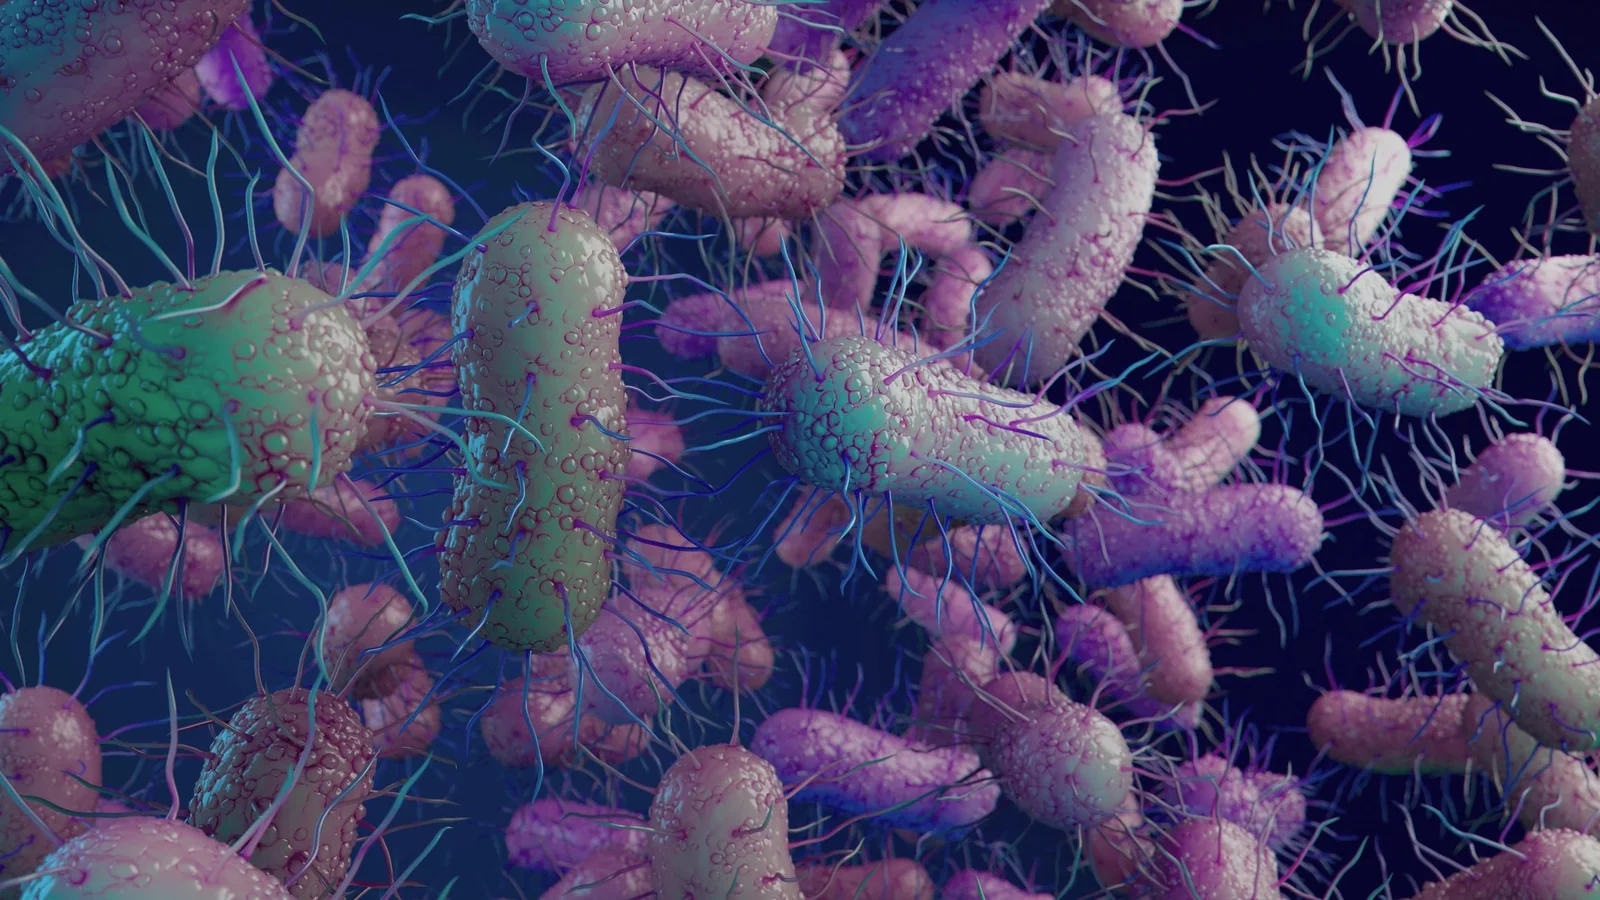
The bacterial flagellum is one of the most efficient and most studied propulsion systems in biology. Its helical shape and rotation are essential to its function: it is a rotating helix, not a beating whip. This mechanism is fundamentally different from eukaryotic cilia and flagella.
2. Structure of the Bacterial Flagellum
The bacterial flagellum is composed of three parts: the basal body (anchored in the membrane), the hook (flexible junction structure) and the helical filament (the propulsive part). The filament is a polymer of flagellin, a protein that self-assembles into a hollow helix about 20 nm in diameter. Its helical shape is determined by the flagellin structure and can change depending on conditions.
3. The Rotary Molecular Motor
The basal body contains a rotary motor powered by the proton gradient (or sodium in some species) across the membrane. This motor can rotate at 100-1000 revolutions per second in both directions. When flagella rotate counterclockwise (viewed from behind), they bundle together and propel the bacterium in a straight line. When some flagella reverse rotation, the bundle disassembles and the bacterium tumbles randomly.
4. Swimming and Chemotaxis
Bacterial swimming alternates between "run" phases (straight swimming) and "tumble" phases (random reorientation). Chemotaxis — the ability to swim toward attractants and away from repellents — is achieved by modulating tumble frequency: the bacterium tumbles less often when moving toward an attractant, producing net movement in the right direction.
5. Conclusion
The bacterial flagellum is a remarkable example of evolved molecular engineering: a nanometric rotating helix powered by an electrochemical gradient, capable of efficient propulsion in a viscous medium at low Reynolds number. Its helical shape is functionally essential, not ornamental.
The relation to the site’s thesis is precise: a rotary motor turning a helix into thrust may share geometry, dynamics, or representation with another family of phenomena, but these levels are not identical. Comparison becomes scientific when it names the proposed shared mechanism, the variables that differ, and the test that could distinguish them.
The relation to the site’s thesis is precise: a rotary motor turning a helix into thrust may share geometry, dynamics, or representation with another family of phenomena, but these levels are not identical. Comparison becomes scientific when it names the proposed shared mechanism, the variables that differ, and the test that could distinguish them.
The relation to the site’s thesis is precise: a rotary motor turning a helix into thrust may share geometry, dynamics, or representation with another family of phenomena, but these levels are not identical. Comparison becomes scientific when it names the proposed shared mechanism, the variables that differ, and the test that could distinguish them.
The relation to the site’s thesis is precise: a rotary motor turning a helix into thrust may share geometry, dynamics, or representation with another family of phenomena, but these levels are not identical. Comparison becomes scientific when it names the proposed shared mechanism, the variables that differ, and the test that could distinguish them.
The relation to the site’s thesis is precise: a rotary motor turning a helix into thrust may share geometry, dynamics, or representation with another family of phenomena, but these levels are not identical. Comparison becomes scientific when it names the proposed shared mechanism, the variables that differ, and the test that could distinguish them.
Approaching the phenomenon without confusing image and mechanism
The concrete starting point is a rotary motor turning a helix into thrust. A bacterial flagellum is a helix driven by a molecular motor. Rotation of the filament in a viscous fluid creates thrust while the cell body receives an opposite reaction. The cell does not swim like a fish at large scale: it exploits low-Reynolds-number mechanics. This first distinction matters because a winding form can be a trajectory, a structure, a projection, or simply a graphical convention.
The model that makes comparison testable
The relation among torque, rotation rate, helical pitch, and force depends on geometry and hydrodynamic resistance. At this scale, inertia fades rapidly and viscous forces dominate. A helix is functional because it converts rotation into translation in a particular medium. [1] The model is not the object: it is a description whose assumptions must remain visible.
An example, then its counter-example
In some bacteria, reversing motor rotation changes flagellar bundle organization and swimming behavior. “Run and tumble” paths result from motor states and responses to chemical gradients. Helical shape alone is therefore insufficient to predict cell behavior. The counter-example is as instructive as the example: it shows which variable is missing when moving from one domain to another.
What can actually be measured
A useful visualization shows filament, axis, rotation direction, and opposing forces. It may vary pitch and viscosity but must signal that it is a model. Real biological parameters are measured separately through microscopy or trajectory tracking. A quantitative figure must distinguish published data, theoretical calculation, simulation, and conceptual diagram.
Decomposing variables instead of following the silhouette
To understand a rotary motor turning a helix into thrust, separate at least the variable that rotates, the one that changes scale, and the one that transports information or matter. A bacterial flagellum is a helix driven by a molecular motor. Rotation of the filament in a viscous fluid creates thrust while the cell body receives an opposite reaction. The cell does not swim like a fish at large scale: it exploits low-Reynolds-number mechanics. A global form can remain stable while its components are replaced; conversely, a trajectory can change shape without a new local mechanism.
The counter-example that protects the reasoning
Helix and spiral share winding, but the helix is three-dimensional and coupled to a motor. This is a clear example of functional convergence: geometry is selected or retained because it efficiently converts rotation into displacement. We therefore cannot conclude from an image alone. We must ask which observation would falsify the hypothesis, then keep negative results in the comparison. This discipline is especially important when several models produce a similar outline.
A reproducible method
A useful visualization shows filament, axis, rotation direction, and opposing forces. It may vary pitch and viscosity but must signal that it is a model. Real biological parameters are measured separately through microscopy or trajectory tracking. To make the result checkable, preserve parameters, units, resolution, initial conditions, and calculation method. An interactive visualization should also provide a readable initial state and a reset control; otherwise readers see an output without understanding its dependencies.
Open questions
The model explains the relation among torque, rotation rate, helical pitch, and force depends on geometry and hydrodynamic resistance. at this scale, inertia fades rapidly and viscous forces dominate. a helix is functional because it converts rotation into translation in a particular medium. [1] but does not answer questions at every scale. We still need to determine how initial conditions, perturbations, and system boundaries alter the pattern. This is where research begins: not by adding an analogy, but by formulating a prediction that could be measured.
Limits and scope of the analogy
Helix and spiral share winding, but the helix is three-dimensional and coupled to a motor. This is a clear example of functional convergence: geometry is selected or retained because it efficiently converts rotation into displacement. [2]
Where the spiral is — and where it is not
The relation to the site’s thesis is precise: a rotary motor turning a helix into thrust may share geometry, dynamics, or representation with another family of phenomena, but these levels are not identical. Comparison becomes scientific when it names the proposed shared mechanism, the variables that differ, and the test that could distinguish them.
References
- [1]Lorenz, Edward N.. (1963). Deterministic Nonperiodic Flow. Journal of the Atmospheric Sciences. DOI: 10.1175/1520-0469(1963)020<0130:DNF>2.0.CO;2
- [2]Watson, J. D.; Crick, F. H. C.. (1953). Molecular Structure of Nucleic Acids. Nature. DOI: 10.1038/171737a0