1. Introduction
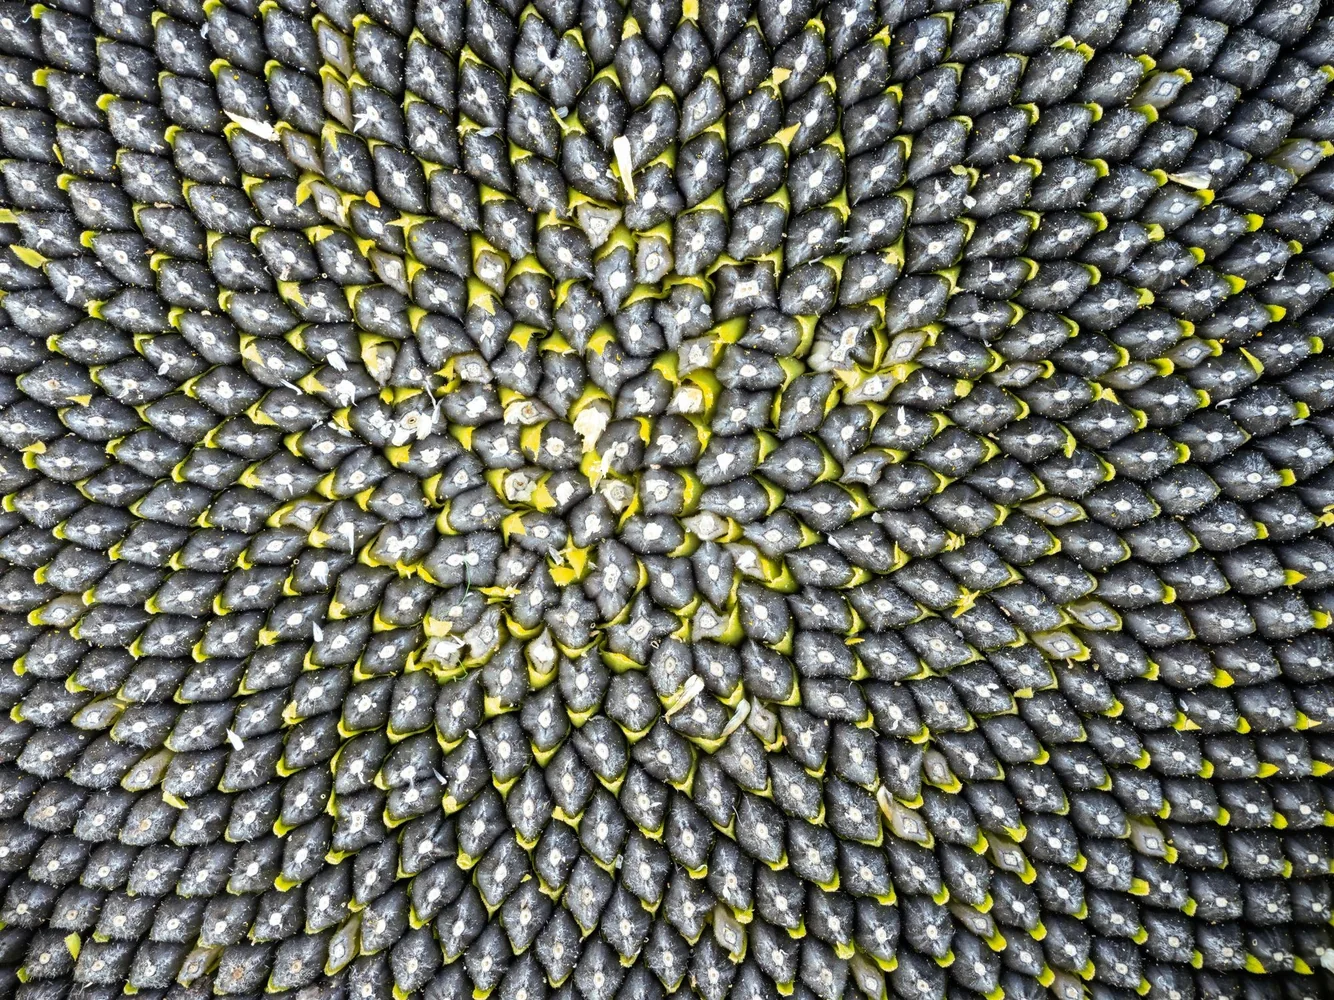
A sunflower typically has 34 spirals in one direction and 55 in the other — two consecutive Fibonacci numbers. A pine cone has 8 and 13. This is not coincidence or cosmic design: it is the mechanical consequence of how plants produce their organs.
2. The Apical Meristem
The apical meristem is a zone of undifferentiated cells at the tip of the stem. This is where primordia form — the rudiments of future leaves, petals or seeds. Each new primordium appears in the most available space, furthest from the primordia already in place.
This principle of spatial inhibition — each organ repels the next ones — is sufficient to generate spiral patterns without any global plan being necessary. The spiral emerges from purely local rules.
3. The Golden Angle
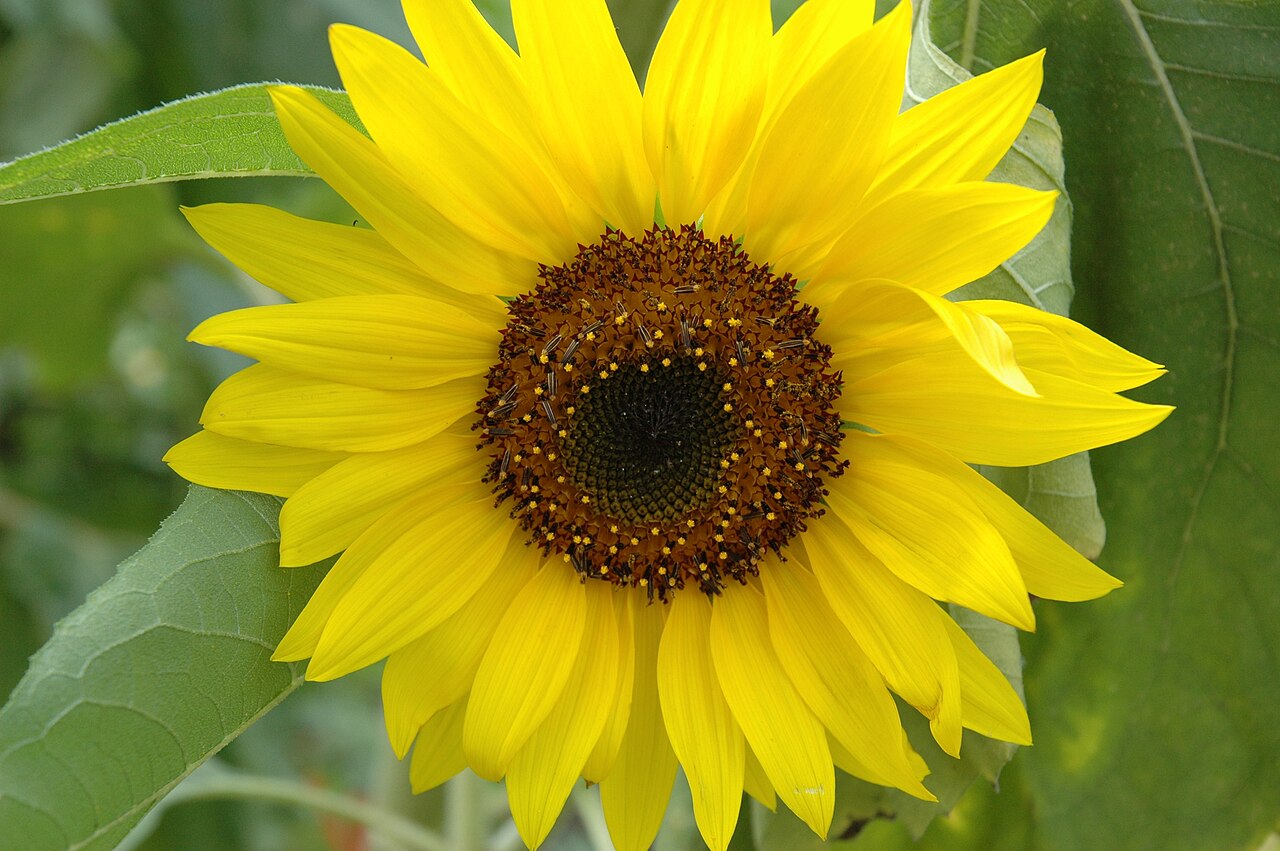
The golden angle is approximately 137.508°. It is the angle that divides a circle in the ratio of the golden number φ ≈ 1.618. If each new primordium appears at 137.508° from the previous one, no radial direction is ever overcrowded: the distribution is maximally uniform.
This angle is irrational in the deepest sense: it is the least well approximable by simple rational fractions. This is precisely what guarantees the absence of privileged directions.
4. Fibonacci and Phyllotaxis
When you trace the visible spirals in a sunflower, you get two families of spirals winding in opposite directions. Their numbers are always two consecutive Fibonacci terms: (1,1), (1,2), (2,3), (3,5), (5,8), (8,13), (13,21), (21,34), (34,55), (55,89)...
This link with Fibonacci follows directly from the golden angle: the best rational approximations of φ are successive Fibonacci ratios. The visible spirals correspond to the directions where primordia align most closely.
5. Mechanical Models
Several physical models reproduce phyllotaxis. The Douady and Couder model (1992) uses magnetic drops deposited on a rotating disk: they repel each other and spontaneously organize according to the golden angle. The Mitchison model (1977) uses auxin gradients — a plant hormone — to simulate inhibition between primordia.
6. Reading parastichies without confusing cause and appearance
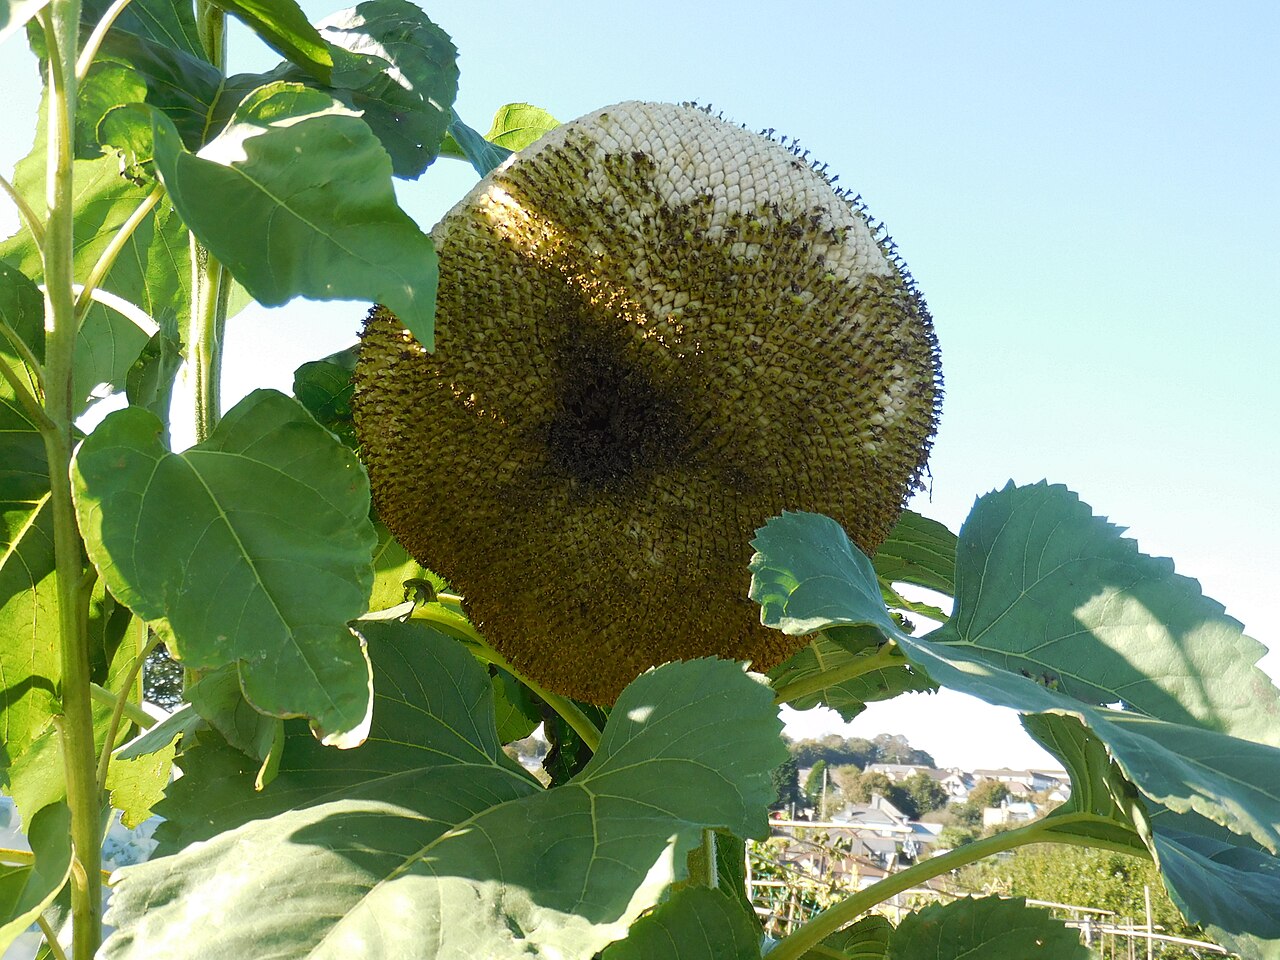
The curved lines followed by the eye on a pine cone or flower head are parastichies. They connect neighboring organs in the final pattern, but the plant does not first draw these spirals and then place organs on them. The generative order is a temporal sequence of primordia; spiral families become visible afterward when several geometric neighbors are compared. The number of parastichies therefore depends on developmental stage, the definition of neighborhood, and how the surface has expanded.
This distinction explains why two photographs of the same kind of plant may emphasize different pairs, such as 34/55 or 55/89. These integers describe robust local organization, not an immutable numerical signature of the species. Counting requires a sufficiently complete image, a well-identified center, and an explicit convention for interrupted or branching lines.
7. Auxin, polar transport, and the creation of a new primordium
At the meristem, auxin does not act as paint marking a predefined location. Membrane transporters, including PIN1, orient flows between cells. Local auxin maxima emerge in the outer layer; when a maximum reaches the conditions required for initiation, a new primordium forms. Experiments that disrupt polar transport alter or stop initiation, while local auxin application can trigger an organ. [1]
An existing primordium then redistributes the transport field and reduces the probability that another will appear too close. The pattern thus results from a loop: transport, accumulation, initiation, and modification of transport. Cellular models show that such a loop can produce stable phyllotaxis and transitions among opposite, decussate, and spiral arrangements without a central clock dictating every angle. [2]
8. The golden angle is a geometric attractor, not an instruction
Saying that organs are separated by about 137.5 degrees is a useful description, but it does not reveal the mechanism by itself. In iterative systems where new elements are added near a growing front and repel one another at short range, several rational organizations are initially possible. As relative growth rate changes, arrangements reorganize and may converge toward a divergence close to the golden angle.
Douady and Couder reproduced Fibonacci families in a physical experiment and simulation where successive elements interacted locally. Their result shows that phyllotactic order can emerge through self-organization. It does not prove that every plant uses exactly the same physical mechanism; it establishes instead that no mystical proportion is required to obtain the observed order. [3]
9. From Vogel’s model to a measurable figure
Vogel’s model places the nth point at angle = nα and radius . The term gives approximately constant area per point because disk area grows as . If α is close to the golden angle, points avoid simple radial alignments for a long time and fill the disk regularly. This model constructs a geometry, not living tissue. [4]
It nevertheless serves as a conceptual laboratory: changing α slightly produces radial lines, empty sectors, or new parastichy families. This separates three questions that are often conflated: how to distribute points on a disk, how a meristem selects the next site, and how later growth deforms the pattern. Visual resemblance among their outcomes does not make these three problems identical.
10. What must be measured to test an explanation
A rigorous study follows primordia through time rather than merely counting spirals on a mature organ. It measures divergence angle, the plastochron between initiations, meristem size, transporter position, and displacement caused by growth. Genetic, chemical, or mechanical perturbations can then separate correlation from causation.
Phyllotaxis therefore illustrates a convergence of levels: local cellular dynamics produces an initiation sequence, that sequence becomes a geometric network, and the network reveals countable spirals. Fibonacci equations summarize some regularities of this network; they do not replace meristem biology or the growth history that built it.
11. Variation, exceptions, and the model’s scope
Not every plant displays spiral Fibonacci phyllotaxis. Leaves may be opposite, whorled, or distributed in irregular patterns, and one individual can change regime during development. Damage, mutations, and changes in meristem size can trigger transitions. A general model must therefore explain not only frequent regularity but also stable alternatives and the possibility of moving from one to another.
Even when Fibonacci numbers appear, they do not directly measure a molecule or force. They emerge from ranking neighborhoods in a lattice produced by growth. The defensible conclusion is precise: some local dynamics make these pairs highly probable and robust. That claim is scientifically more informative than the absolute statement that nature “follows” one universal numerical sequence.
12. Synthesis
A phyllotactic spiral is therefore neither a prior blueprint nor a graphical accident. It is a geometric reading of sequential development. Hormones and their transporters organize initiation sites; growth displaces those sites; neighborhoods reveal parastichies; and some dynamical regimes favor Fibonacci pairs. Each level has its own measurements and uncertainties, but their predictions can be connected. The scientific explanation lies in that connection rather than in assigning causal power to one number.
6. Conclusion
Phyllotaxis illustrates how simple local rules — each new organ avoids its neighbors — produce complex and mathematically precise global patterns. The golden ratio and Fibonacci are not the cause: they are the inevitable consequence of space optimization in a continuously growing system.
References
- [1]Reinhardt, Didier et al.. (2003). Regulation of Phyllotaxis by Polar Auxin Transport. Nature, 426, p. 255–260. DOI: 10.1038/nature02081. https://www.nature.com/articles/nature02081
- [2]Smith, Richard S. et al.. (2006). A Plausible Model of Phyllotaxis. Proceedings of the National Academy of Sciences, 103(5), p. 1301–1306. DOI: 10.1073/pnas.0510457103. https://pmc.ncbi.nlm.nih.gov/articles/PMC1345713/
- [3]Douady, Stéphane; Couder, Yves. (1992). Phyllotaxis as a Physical Self-Organized Growth Process. Physical Review Letters, 68(13), p. 2098–2101. DOI: 10.1103/PhysRevLett.68.2098. https://journals.aps.org/prl/abstract/10.1103/PhysRevLett.68.2098
- [4]Vogel, Helmut. (1979). A Better Way to Construct the Sunflower Head. Mathematical Biosciences, 44(3–4), p. 179–189. DOI: 10.1016/0025-5564(79)90080-4. https://doi.org/10.1016/0025-5564(79)90080-4