1. Introduction
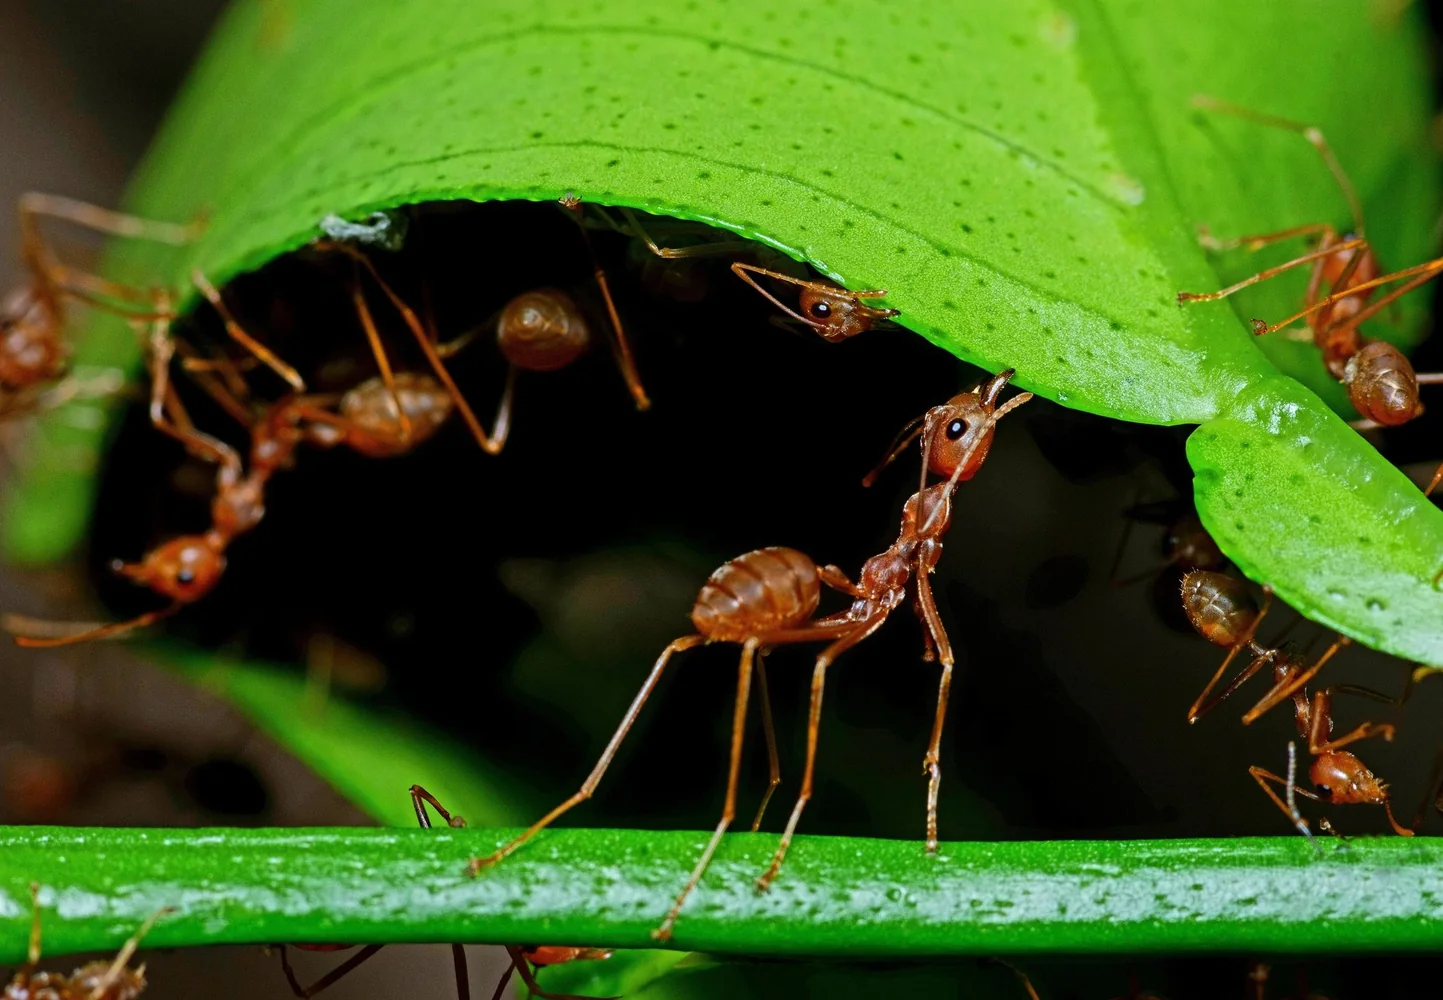
An ant colony can find the shortest path between its nest and a food source, distribute its workers among different tasks according to need, and build nests of remarkable architectural complexity — all without a leader, without a global plan, and without direct communication between individuals. This apparent paradox between the simplicity of individuals and the sophistication of the collective is at the heart of social insect biology and complex systems theory.
Stigmergy is one of the mechanisms that explain this coordination. The term designates a form of indirect coordination in which the actions of an agent modify the environment, and these modifications influence the actions of subsequent agents. The environment thus becomes a shared external memory that coordinates collective behavior without requiring direct communication or a global representation.
2. Definition and History of the Concept
The term stigmergy was introduced by French biologist Pierre-Paul Grassé in 1959 to describe the coordination of construction in termites. Grassé observed that termites did not seem to follow a pre-established plan, but responded to the current state of the construction. A deposit of material became a stimulus for a neighboring deposit; the emerging structure guided subsequent actions. Grassé coined the term from the Greek <em>stigma</em> (mark, sign) and <em>ergon</em> (work): work guided by marks.
Grassé's definition was broadened and refined by later researchers. Eric Bonabeau, Marco Dorigo, and Guy Theraulaz distinguished two types of stigmergy: quantitative stigmergy (the quantity of a trace, such as pheromone concentration, guides behavior) and qualitative stigmergy (the nature or form of a trace guides behavior). This distinction matters because the mechanisms and properties of the two types differ.
Stigmergy is a special case of a more general phenomenon: environment-mediated coordination. It is distinct from direct communication (one agent sends a signal to another agent) and from coordination by global rules (all agents follow the same algorithm without interaction). In stigmergy, coordination emerges from the interaction between agents and their shared environment.
3. Pheromones and Path Optimization

The most studied example of quantitative stigmergy is path optimization by ants. When an ant explores its environment, it deposits a pheromone trail along its path. If it finds food and returns to the nest, it reinforces this trail. Other ants, attracted by pheromones, tend to follow more concentrated trails. A shorter path is traveled more quickly, allowing the ant to make more round trips per unit of time and deposit more pheromones. Positive feedback progressively selects the shortest path.
This mechanism was demonstrated experimentally by Deneubourg et al. (1990) with the "two-bridge experiment": ants placed between their nest and a food source with two paths of different lengths progressively choose the shorter path. Pheromone evaporation is essential: without it, the system would lock onto the first path explored, regardless of its length. Evaporation introduces a form of forgetting that maintains adaptive capacity.
It is important to note that this mechanism does not always produce the mathematically optimal path. It produces a good solution under normal conditions, but can lock onto a suboptimal path if conditions change rapidly or if the colony is too small to explore sufficiently. The robustness of the mechanism depends on the ratio between the pheromone deposition rate, the evaporation rate, and the colony size.
4. Termite Construction: Architecture Without an Architect
The termite mounds of certain African species (notably <em>Macrotermes bellicosus</em> and <em>Macrotermes michaelseni</em>) are among the most complex constructions in the animal kingdom. They can reach several meters in height, contain millions of individuals, and feature sophisticated ventilation systems that maintain temperature and CO₂ levels within narrow ranges. These structures are built by individual termites who cannot perceive the global structure and do not follow a central plan.
The mechanism proposed by Grassé and confirmed by later studies is an example of qualitative stigmergy. A termite deposits a ball of earth impregnated with pheromones. This ball attracts other termites who deposit their balls nearby. A pillar begins to form. When two neighboring pillars reach a certain height, termites begin to incline them toward each other, forming an arch. This behavior is triggered by the shape of the existing structure, not by a central instruction.
Computational models of termite mound construction (Theraulaz and Bonabeau, 1995; Turner, 2000) have reproduced structures resembling real mounds using simple local rules. These models show that architectural complexity can emerge from simple rules applied locally, without requiring a global representation. They also show that the structures produced depend strongly on the parameters of the local rules and on environmental conditions (humidity, temperature, air currents).
The shape of termite mounds varies considerably by species and environment. Some species build cylindrical towers, others mushroom-shaped structures, others complex underground nests. The spiral can appear in certain architectures (helical galleries, spiral structures), but it is not a universal property of stigmergic constructions. Each architecture is the result of local rules specific to the species and environmental conditions.
5. Human and Digital Stigmergy
The concept of stigmergy has been extended to human and digital systems. In these contexts, the "traces" are not pheromones but cultural artifacts, documents, data, or states of computer systems. Human stigmergic coordination is ubiquitous: a shared whiteboard, a code repository (Git), a Wikipedia page, an online discussion thread — all are environments modified by the actions of participants that guide subsequent actions.
Wikipedia is a particularly striking example. Millions of articles have been created and improved by contributors who do not know each other and do not coordinate directly. Each modification leaves a trace (the modified article, the revision history) that guides subsequent modifications. The overall quality of the encyclopedia emerges from these local interactions, without a central editor overseeing each article.
Digital stigmergy has different properties from biological stigmergy. Digital traces do not evaporate (unless explicitly deleted), can be copied and distributed instantly, and can be read by remote agents. These differences modify coordination dynamics: the persistence of traces can create stronger lock-in effects than in biological systems; instant distribution can accelerate convergence toward common solutions.
6. Ant Colony Algorithms
Ant Colony Optimization (ACO) algorithms were developed by Marco Dorigo from 1992 onward as a family of optimization methods inspired by ant behavior. In these algorithms, virtual agents (artificial ants) explore a solution space by depositing virtual traces (digital pheromones) on the solutions they visit. The quality of a solution determines the amount of pheromones deposited; evaporation maintains the diversity of exploration.
ACO algorithms have been successfully applied to many combinatorial optimization problems: the traveling salesman problem, routing in telecommunications networks, task scheduling, electronic circuit design. They are particularly effective for problems where the solution space is large and discrete, and where local heuristics can guide exploration.
The convergence of ACO algorithms is well studied theoretically. Under certain conditions (appropriate evaporation rate, sufficient number of agents), they converge toward near-optimal solutions. But as with biological ants, this convergence is not guaranteed in all cases, and the algorithm parameters must be tuned to the problem. The biological metaphor is useful for intuition, but mathematical rigor requires independent analysis.
7. Limits of the Concept and Link to the Spiral
Stigmergy is a powerful concept but has its limits. It describes a coordination mechanism, not a universal property of all collective systems. Not all collective behaviors are stigmergic: some require direct communication, others rely on genetically programmed rules without environmental interaction. Stigmergy is a partial explanation that must be complemented by other mechanisms to account for the complexity of observed collective behaviors.
The link between stigmergy and the spiral is indirect but real. Stigmergy is a mechanism of emergence: complex structures emerge from simple local interactions. The spiral can be one of these emergent structures in certain contexts (helical termite galleries, spiral ant trajectories under certain conditions), but it is not the necessary result of stigmergy in general. The connection with the "Spirals Everywhere" project lies in the emergence mechanism itself: how simple local rules can produce complex global forms, sometimes including spirals.
What stigmergy illustrates for the project is the convergence between very different domains (insect biology, computer science, social sciences) toward the same abstract mechanism: coordination through environmental modification. This convergence is not due to a common physical law or shared evolutionary origin; it reflects the generality of an organizational principle that can be independently rediscovered in very different contexts.
The environment becomes shared memory
In direct communication, one agent addresses another. In stigmergic coordination, an agent modifies the environment, making a subsequent action more likely there. The trace may persist after its producer leaves. The next agent need not meet the producer or know its intention. This separation between an action and its later consequence is the mechanism to identify, rather than merely comparing a group to a central “intelligence.”
Deneubourg and colleagues’ work on Argentine-ant exploration shows how local trail deposition and following can produce collective organization. The following laboratory is a teaching construction inspired by that principle. It reproduces neither their experiment nor measured pheromone concentrations. To identify the mechanism elsewhere, specify what writes the trace, what reads it and what erases it. [1]
Building a local choice between two paths
At each step, six agents choose between two branches. Choice probability depends on squared trace plus a small background of 0.1, favoring an already marked branch without eliminating exploration. The short path returns one trace unit after two steps; the long path after five. Both start with trace one. The delay difference allows one branch to receive earlier returns and benefit from reinforcement. Choices remain stochastic, with a fixed seed for reproducibility.
The graph shows traces, not real colony counts. Deposits from agents already traveling arrive after their delay and influence later choices. Evaporation changes the balance between accumulation and forgetting. Even when a path dominates, no agent has globally compared all routes. The model also does not guarantee a general optimum and may retain a preference that is no longer useful.
Evaporation sets memory duration
Without new deposits, fraction ρ disappears each step, leaving (1−ρ)ᵗ after t steps. With ρ=0.08, one step retains 92% of the trace; repeated multiplication gives decay, not a subtraction of eight units. All three curves start from the same value to isolate the effect. Persistent memory stabilizes a decision but retains old information; fast forgetting supports adaptation while making information more fragile.
This tension between stability and responsiveness occurs in many coordination systems, but every analogy needs its own mechanism checked. A collaborative page retains changes under editorial rules; it does not automatically evaporate like pheromone. Calling something stigmergy does not transfer ant parameters to human systems. The schematic supplies questions about local memory, not a universal equation for collective intelligence.
Closing a path reveals the role of forgetting
In the final experiment, the short branch becomes inaccessible at step fifty. New departures must use the long branch, while already pending short-branch deposits still arrive before fading. The displayed probability drops to zero because access is closed, not because agents anticipated the obstacle. Old trace can remain high for several steps: information stored in the environment is not automatically current.
The test separates a choice rule, an access constraint and an erasure mechanism. Assessing real adaptation would require separate measurements of detection delay, trace renewal and performance recovery. A curved trail or spiral walk is not required for stigmergy: the mechanism concerns environmental mediation. Conversely, an attractive spiral pattern alone does not demonstrate collective memory. [1]
References
- [1]Deneubourg, J.-L.; Aron, S.; Goss, S.; Pasteels, J. M.. (1990). The self-organizing exploratory pattern of the argentine ant. Journal of Insect Behavior. DOI: 10.1007/BF01417909. https://link.springer.com/article/10.1007/BF01417909 [accessed 2026-10-19]